Rice (Oryza sativa L.) is one of the major cereal crops produced in Pakistan and is cultivated on an area of 2,900,600 hectares with a production of 11,174,700 tons (FAO, 2017). As a staple food, its consumption exceeds 100 kg per capita annually in most of the Asian countries (Seck et al., 2012). Several biotic and abiotic constraints limit the yield and quality of rice. Among biotic constraints, plant-parasitic nematodes are an emerging threat to rice production. Root-knot nematodes (RKNs) are the most destructive plant-parasitic nematodes in upland, lowland, and deep-water rice cultivation systems (Panwar and Rao, 1998; Bridge et al., 2005). RKNs possess the ability to penetrate the roots, induce root galling, suppress plant defense mechanisms, hijack the plant’s metabolic system, and establish giant cells for the sake of their own benefit (Kyndt et al., 2014; Ali et al., 2017a, 2017b, 2018). As an outcome, plants gradually lose vigor, ultimately leading to substantial yield loss (Bridge et al., 2005; Win et al., 2015; Ali et al., 2015). Among various RKNs, Meloidogyne graminicola (Golden and Birchfield) has emerged as the most serious pest of rice (Mantelin et al., 2017). M. graminicola was first reported in Pakistan by Munir and Bridge (2003) during a survey of rice fields of Sheikhupura, Punjab, Pakistan. The subtropical climate of Pakistan and warm sandy soils are favorable for the development and reproduction of RKNs (Khattak, 2008). But plant-parasitic nematodes in these regions have received little attention in the past, and only a few surveys have been conducted to estimate their prevalence and incidence (Kafi, 1963; Ahmad and Khan, 1973; Saeed and Ashrafi, 1973; Khan et al., 2005; Zarina and Shahina, 2010; Anwar and McKenry, 2012). All varieties of rice grown in South Asian and Southeast Asian countries, whether upland or lowland, have exhibited susceptibility to M. graminicola (Padgham et al., 2004; Das et al., 2011; Win et al., 2013). Currently, there is little information about the association of M. graminicola with rice in Pakistan.
Compared with other phytopathogens, nematodes are difficult to control because they attack belowground parts of plants, resulting in reduced growth and yield loss (Williamson and Hussey, 1996). Moreover, nematodes are polyphagous pests that attack over 5,500 plant species, including several economically important crops (Moens and Perry, 2009; Ali et al., 2015; Ali et al., 2019). Successful control of Meloidogyne species can only be achieved by rapid and accurate identification of the nematode. Traditional techniques of nematode identification based on morphological features (Eisenback, 1985) are challenging because they are laborious and require extensive training and expertise. Historically, RKNs have been identified based primarily on morphological features. Currently, there is no information available about the molecular identification of Meloidogyne spp. in Pakistan, especially in regard to M. graminicola.
Several molecular techniques are available for the identification of Meloidogyne species (Blok and Powers, 2009). Among these techniques, the polymerase chain reaction (PCR) is a sensitive, quick, and accurate tool (Niu et al., 2011). Adam et al. (2007) developed a molecular diagnostic key that uses several molecular approaches to identify seven economically important RKNs that are frequently encountered in diagnostic laboratories. Moreover, with the increase in DNA-based sequencing, the tandem repeat unit segments of the 18 S, ITS1, 5.8 S, ITS2, and 28 S regions of the ribosomal DNA array (rDNA) and mitochondrial DNA (mtDNA) have proved to be efficient diagnostic tools for accurately identifying of RKNs (Landa et al., 2008; Naz et al., 2012).
Accurate identification of M. graminicola, as well as its prevalence and distribution spectra, is fundamental for applying management strategies in the field. Therefore, we used morphological and molecular approaches to identify RKNs in order to determine the distribution, prevalence, and disease intensity of M. graminicola in Chiniot and Faisalabad districts of Central Punjab, Pakistan.
Materials and Methods
Survey and sampling
A survey of rice-growing areas of Faisalabad and Chiniot districts of central Punjab, Pakistan, was conducted during September 2014, 2015, and 2016. Five root samples of rice plants and 1000-ml composite soil samples were collected from each sampling site, preserved in polythene bags, and labeled. The samples were transported to the Nematology Lab, Department of Plant Pathology, University of Agriculture, Faisalabad, for further processing. The roots were gently washed with distilled water to remove adhering soil and plant debris. Nematode prevalence was determined by using the formula of Norton (1978):
Isolation and morphological identification of M. graminicola
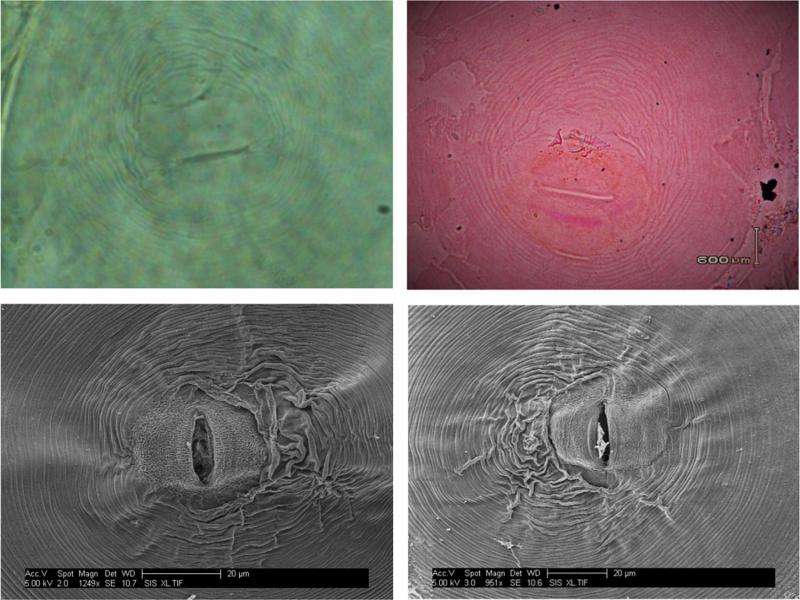
Second-stage juveniles (J2s) of M. graminicola were isolated from rice roots. The root samples from each field were pooled, chopped into pieces, and mixed thoroughly. Three subsamples of 5-g roots were taken, and juveniles were isolated from infected roots using the Baermann funnel method and collected in a beaker. Nematode extraction from soil samples was carried out using Whitehead’s tray method (Whitehead and Hemming, 1965). Soil samples were mixed thoroughly, and a 100-ml composite sample was placed in a plastic bucket and 1–2 liters of water were added. Plant debris, heavy soil particles, and rocks were drained manually. The supernatant was sieved through a 50-mesh-size sieve in a separate bucket. The procedure was repeated by adding 1,000-ml water again and agitated properly. After that, the suspension was left to settle and poured again into another basket using a 100-mesh sieve. The process was repeated twice again using 250- and 325-mesh sieves. The final suspension was transferred to a 500-ml beaker and the supernatant was allowed to settle for one hour. Three subsamples of 2 ml each were taken and examined in a counting dish. Second-stage juveniles (J2) were counted using a stereomicroscope (Olympus SZ2-ILGB). Mature females of M. graminicola were identified based on micrographs of the internal and external perineal patterns (Jepson, 1987). Stained hooked gall tissues were teased apart with a pointed needle to separate mature females. The neck region of individual nematodes was excised, and the posterior part was dipped in 45% lactic acid solution to remove body tissues. The perineal patterns were trimmed and transferred on a transparent glass slide in a glycerin drop. External views of the perineal patterns were visualized using scanning electron microscopy (SEM) at Brigham Young University, Provo Utah, USA. Accordingly, specimens were dehydrated via ascending ethanol series prior to critical point drying. The animals were then mounted on stubs and gold-sputtered. Micrographs were recorded via Helios Nanolab 600 SEM (Thermo-Fisher Scientific, Hillsborough, USA).
Statistical analysis
Data were subjected to statistical analysis using Statistix (Ver. 8.1). The experimental design for the analysis of galling index, juveniles/soil sample, juveniles/root sample, stylet, and non-stylet-bearing nematodes was by a completely randomized block design with treatment means separated using a LSD test at P = 0.05.
DNA extraction
Isolates derived from single egg masses were used to extract DNA. Twenty larvae were picked, rinsed thrice with sterile distilled water, transferred to a microcentrifuge tube, and crushed in 500 µL of SDS extraction buffer containing Tris–HCl (1 M, pH 7.5), EDTA (0.5 M, pH 8.0), SDS (10% w/v), and dd H2O with a grinding plastic stick (Mitkowski et al., 2003). Proteins in the solution were digested by adding 20 µL proteinase K, 100 µg ml−1. Later, 500 µL of phenol (25:24:1, phenol/chloroform/isoamyl alcohol) was added and vortexed briefly. The tube was centrifuged at 14,000 rpm for 5 min and the supernatant was collected and transferred to another sterile microcentrifuge tube. Sodium acetate (3 M), 50 µL and ice-cold isopropanol, 500 µL, were added to the supernatant, vortexed gently, and centrifuged at 14,000 rpm for 5 min. The supernatant was discarded to save the pellet. Five-hundred µL of ethanol (96%) was added to the pellet and centrifuged for 3 min at 13,000 rpm. The supernatant was discarded again, and the pellet air-dried in a laminar flow chamber for 2 hr. DNA was dissolved in 30 µL of TE buffer (1 ml of 1 M Tris base (pH 8.0) and 0.2 ml of EDTA (0.5 M), dd H2O) and stored at –20°C until required for PCR reactions.
Internal transcribed spacer region (ITS) amplification
The PCR reaction mixture was prepared by using 10 µL of 10X PCR buffer, 2-µL dNTPs (10 mM), 2-µL forward primer (10 µM), 2-µL reverse primer (10 µM), 2-µL template DNA (> 50 ng), 1-µL Taq polymerase, and 81-µL ddH2O, for a total reaction volume of 100 µL. PCR reactions were carried out in a thermal cycler (BIO-RAD T100TM) under the following conditions: (1) predenaturation at 94 °C for 5 min, (2) denaturation at 94°C for 1 min, (3) annealing at 64°C for 1 min, (4) extension at 72°C for 1 min, (5) 35 cycles of this process, and (6) final extension at 72°C for 5 min. The sequences of primers used for amplification of the internal transcribed spacer region are 1) forward primer rDNA2 (5’–TTGATTACGTCCCTGCCCTTT–3’) (Vrain et al., 1992) and reverse primer rDNA1. 5.8 s (5’–ACGAGCCCGAGTGATCCACCG–3’) (Cherry et al., 1997). Primers were synthesized by Sigma Genosys Inc, St. Louis, MO, USA.
Gel electrophoresis and sequencing
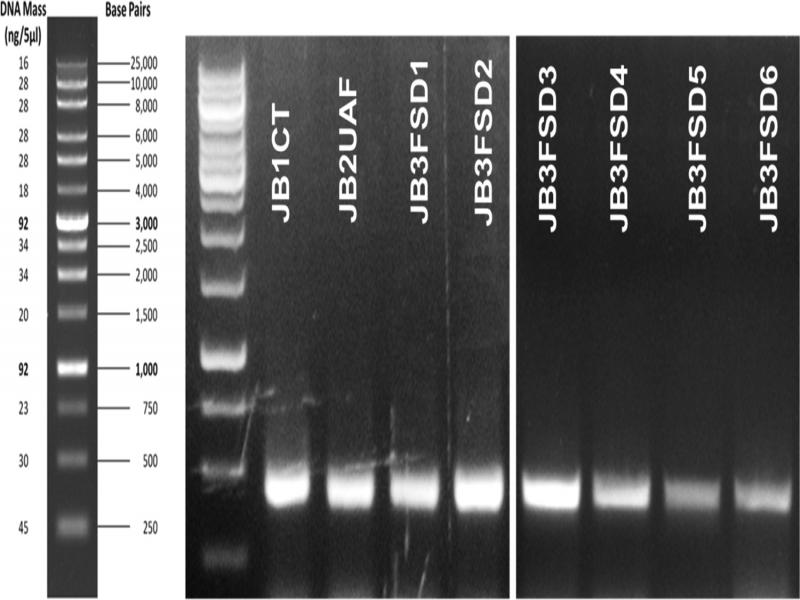
The amplified PCR product was viewed on a gel stained with ethidium bromide under a UV transilluminator. DNA was excised from the gel and purified for sequencing using quick Gel Extraction Kit (Qiagen Gel Extraction Kit, Qiagen, Hilden, Germany). Purified DNA was sent for sequencing to L.G.C. Genomics, Germany, or the DNA sequencing center at Brigham Young University, Provo, Utah, USA.
Phylogenetic analysis
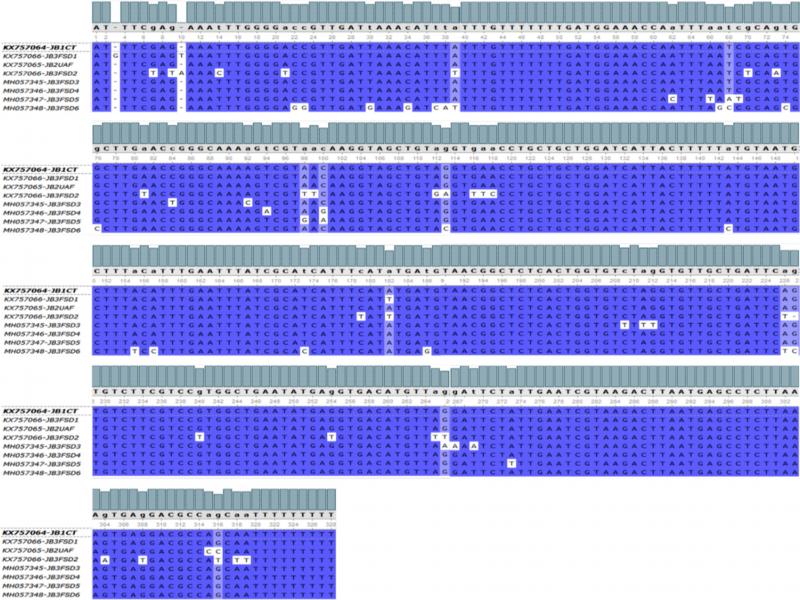
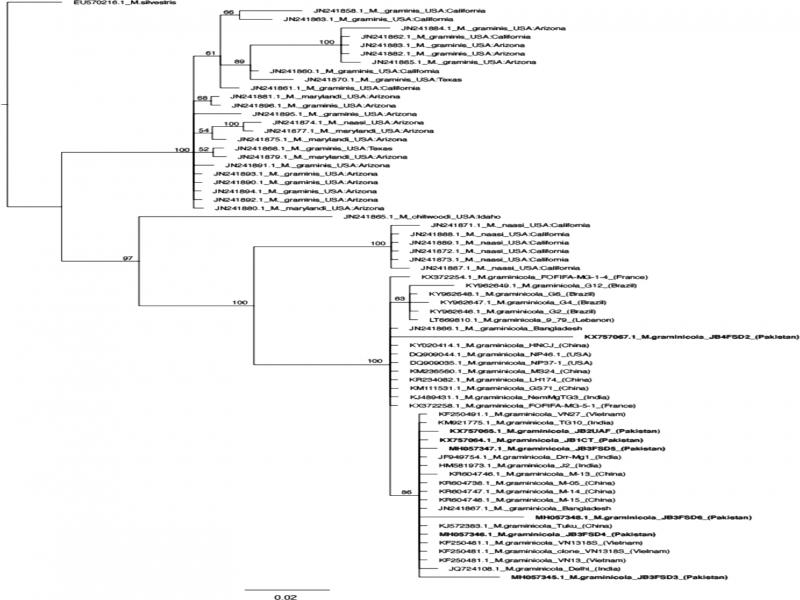
Due to the high degree of interspecific variation in nucleotide sequences of nematodes (Hu and Gasser, 2006), the deduced internal transcribed spacer region sequences were used for phylogenetic study. The ITS sequences of the eight isolates were used to query the most similar curated sequences on GenBank by performing open-nucleotide BLAST (Basic Local Alignment Search Tool, Camacho et al., 2009). The nearest matches as well as those from closely related species of Meloidogyne (McClure et al., 2012) were downloaded from GenBank and used for subsequent phylogenetic analysis. Multiple-sequence alignment was generated using MUSCLE (Edgar, 2004). The alignment settings included optimization of profile-dependent parameters. Sequences were first grouped by similarity with anchor optimization. Iteration 1 = kmer4_6 with pctid_kimura for subsequent interactions using the UPMGB clustering method and pseudo-tree rooting. CLUSTALW was used for the distance weighting scheme, with 32-base anchor spacing and 24-base minimum diagonals. Bayesian analyses were carried out using MrBayes 3.2.6 (Huelsenbeck and Ronquist, 2001). A general time-reversible model of sequence evolution with four categories of gamma rate variation was chosen as the optimal model of sequence evolution as per Posada and Crandall (1998). Bayesian analysis was initiated with a random starting tree with four heated chains of chain length 1,100,000, burn-in length of 100,000, and subsampling frequency of 200. Branch lengths were unconstrained.
Results
Prevalence of M. graminicola
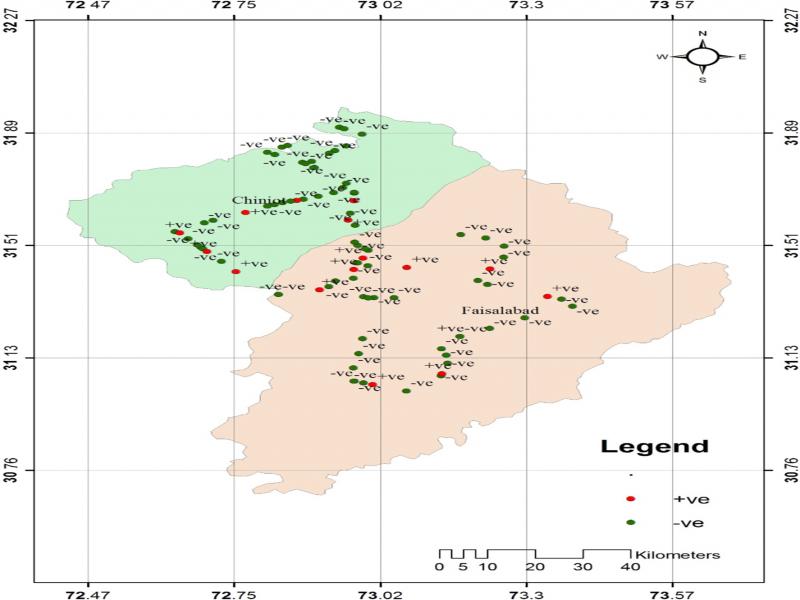
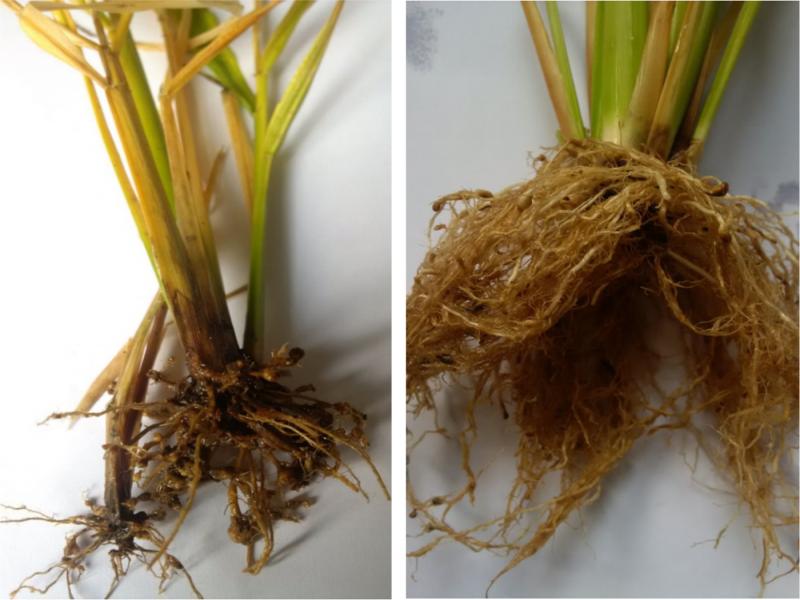
The field survey data during the rice cropping season of 2014, 2015, and 2016 indicated that both districts Chiniot and Faisalabad have M. graminicola infestation during all the seasons. The GPS coordinates for each sample were used to plot the presence and absence of M. graminicola at the sampled sites in Faisalabad and Chiniot (Figure 1). The prevalence of M. graminicola at forty surveyed locations of Chiniot and Faisalabad is given in Tables 1 and 2. Maximum prevalence of M. graminicola (22.5 and 27.5%) was observed in Chiniot and Faisalabad, respectively, during the rice-growing season of 2016, while the minimum prevalence (17.5 and 20%, respectively) was recorded in Chiniot and Faisalabad during the cropping season of 2014. During 2014 to 2016 at Chiniot among 40 surveyed locations, the presence of M. graminicola was observed at 7, 8, and 9 locations respectively. Similarly, 40 locations were surveyed in Faisalabad during 2014–2016, and M. graminicola prevalence was recorded at 8, 10, and 11 locations, respectively. M. graminicola showed typical hook-shaped galls on rice roots that are a characteristic feature of M. graminicola infection (Figure 2).
Table 1.
Prevalence of M. graminicola in Chiniot district.
| Prevalence | |||||||
|---|---|---|---|---|---|---|---|
| Sr # | Locations | Elevation | Latitude | Longitude | 2014 | 2015 | 2016 |
| 1 | 133 J.B. | 178 V | 31.57931 | 072.97683 | − | − | − |
| 2 | 134 J.B. | 173 V | 31.59705 | 072.96338 | + | + | + |
| 3 | 223 J.B. | 169 V | 31.62043 | 072.96727 | − | − | − |
| 4 | Moza Rajoya | 176 R | 31.66198 | 072.97448 | + | + | + |
| 5 | M.Thattian | 184 R | 31.68778 | 072.97489 | − | − | − |
| 6 | M. Johdpur | 180 R | 31.69026 | 072.97472 | − | − | − |
| 7 | Ahmad Nagar | 182 R | 31.77321 | 072.89966 | − | − | − |
| 8 | Ahmad Pur | 187 R | 31.79090 | 072.87729 | − | − | − |
| 9 | M. kanwewala | 183 R | 31.81763 | 072.82544 | − | − | − |
| 10 | Moza Judhi | 186 R | 31.82471 | 072.81122 | − | − | − |
| 11 | 202 J.B. | 192 V | 31.84161 | 072.83868 | − | − | − |
| 12 | Kote Qazipur | 190 R | 31.84774 | 072.84970 | − | − | − |
| 13 | Biewal | 187 R | 31.90920 | 072.94682 | − | − | − |
| 14 | Kalowal | 182 R | 31.90423 | 072.95624 | − | − | − |
| 15 | Jand wala | 185 R | 31.88589 | 072.99015 | − | − | − |
| 16 | Pungu Morr | 184 R | 31.84625 | 072.96008 | + | + | + |
| 17 | Moza Johdabad | 183 R | 31.83006 | 072.93907 | − | − | − |
| 18 | M.Hussainabad | 188 R | 31.82157 | 072.92782 | + | + | + |
| 19 | M.Mohsanabad | 178 R | 31.79400 | 072.89456 | − | − | − |
| 20 | Moza Vaisaan | 176 R | 31.78678 | 072.88346 | − | − | − |
| 21 | 241 J.B. | 178 V | 31.72044 | 072.95988 | − | − | − |
| 22 | Moza Bukharian | 177 R | 31.70576 | 072.95381 | − | − | − |
| 23 | Abbas nagar | 180 R | 31.68935 | 72.93636 | − | − | − |
| 24 | Kandiwal | 177 R | 31.67671 | 72.90760 | − | − | − |
| 25 | 241 J.B. | 179 V | 31.66678 | 72.87928 | − | − | − |
| 26 | Thatta Jahania | 177 R | 31.66310 | 72.86660 | + | + | + |
| 27 | Adil wala bangla | 169 V | 31.66029 | 72.85530 | − | − | − |
| 28 | 194 J.B. | 171 V | 31.65541 | 72.83943 | − | − | − |
| 29 | 94 J.B. | 179 V | 31.64864 | 72.82515 | − | − | − |
| 30 | 202 J.B. | 179 V | 31.62264 | 72.77077 | + | + | + |
| 31 | Moza Nitthar | 167 R | 31.59611 | 72.70949 | − | − | − |
| 32 | 254 J.B. | 168 V | 31.58803 | 72.69275 | − | − | − |
| 33 | Jamya abad | 168 T | 31.55409 | 72.64627 | + | + | + |
| 34 | Gondlan wali | 167 R | 31.53430 | 72.66215 | − | − | − |
| 35 | Chenab mills Ltd | 166 C | 31.51384 | 72.67929 | − | − | − |
| 36 | Bhawana city | 170 C | 31.50520 | 72.68622 | − | − | − |
| 37 | 129 J.B. | 172 V | 31.50039 | 72.69027 | − | − | − |
| 38 | 41 J.B. | 165 V | 31.49171 | 72.69737 | − | + | + |
| 39 | 223 J.B. | 169 V | 31.45835 | 72.72484 | − | − | + |
| 40 | Rahmuana | 181 V | 31.42409 | 72.75250 | − | − | − |
| Prevalence | |||||||
|---|---|---|---|---|---|---|---|
| Sr # | Locations | Elevation | Latitude | Longitude | 2014 | 2015 | 2016 |
| 1 | 217 R.B. | 175 V | 31.44325 | 073.00077 | − | − | − |
| 2 | 61 J.B. | 176 V | 31.45346 | 072.97887 | − | − | − |
| 3 | 57 J.B. | 177 V | 31.45328 | 072.98147 | − | − | − |
| 4 | 58 J.B. | 186 V | 31.46937 | 072.99122 | + | + | + |
| 5 | 52 J.B. | 181 V | 31.49570 | 073.00120 | − | − | − |
| 6 | 54 J.B. | 186 V | 31.500394 | 072.99582 | − | − | − |
| 7 | 51 J.B. | 180 V | 31.51203 | 072.98117 | − | − | − |
| 8 | 53 J.B. | 180 V | 31.52299 | 072.97618 | − | − | − |
| 9 | 49 J.B. | 186 V | 31.56101 | 072.98678 | − | − | − |
| 10 | 218 J.B. | 173 V | 31.43074 | 072.97399 | + | + | + |
| 11 | 64 J.B. | 173 V | 31.39198 | 072.93964 | − | − | − |
| 12 | 68 J.B. | 174 V | 31.37310 | 072.92706 | − | − | − |
| 13 | 66 J.B. | 178 V | 31.40154 | 72.97310 | − | − | − |
| 14 | 275 J.B. | 169 V | 31.34735 | 72.83235 | − | − | − |
| 15 | 70 J.B. | 181 V | 31.36304 | 72.90952 | − | + | + |
| 16 | 289 R.B. | 172 V | 31.33934 | 072.99238 | − | − | − |
| 17 | 245 R.B. | 177 V | 31.33586 | 073.01232 | − | − | − |
| 18 | 296 R.B. | 179 V | 31.33620 | 073.04997 | − | − | − |
| 19 | 254 R.B. | 166 V | 31.33576 | 073.00168 | − | − | − |
| 20 | 269 R.B. | 167 V | 31.19880 | 072.99097 | − | − | − |
| 21 | 135 G.B. | 169 V | 31.14848 | 072.98298 | − | − | − |
| 22 | UAF | 179 C | 31.43735 | 073.07427 | + | + | + |
| 23 | Samundari City | 168 C | 31.05557 | 072.97504 | − | − | − |
| 24 | 71 G.B. | 165 V | 31.05584 | 072.97427 | − | − | + |
| 25 | 73 G.B. | 165 V | 31.05005 | 072.99210 | − | − | − |
| 26 | 442 G.B. | 172 V | 31.04441 | 073.00982 | + | + | + |
| 27 | 393 G.B. | 172 V | 31.02308 | 073.07303 | − | − | − |
| 28 | 423 G.B. | 178 V | 31.07426 | 073.13823 | − | − | − |
| 29 | 424 G.B. | 172 V | 31.08084 | 073.14034 | + | + | + |
| 30 | 430 G.B. | 171 V | 31.11562 | 073.15054 | − | − | − |
| 31 | 172 G.B. | 178 V | 31.14319 | 073.14831 | − | − | − |
| 32 | 171 G.B. | 178 V | 31.16456 | 073.13882 | − | − | − |
| 33 | 39 G.B. | 176 V | 31.20585 | 073.17356 | + | + | + |
| 34 | 41 G.B. | 182 V | 31.20572 | 073.17418 | − | − | − |
| 35 | 54 G.B. | 183 V | 31.26873 | 073.29616 | − | − | − |
| 36 | 21 G.B. | 191 V | 31.30716 | 073.38556 | − | − | − |
| 37 | 205 R.B. | 186 V | 31.43253 | 073.23050 | + | + | |
| 38 | 66 G.B. | 181 V | 31.34015 | 073.33852 | + | + | + |
| 39 | 216 R.B. | 183 V | 31.38091 | 073.22599 | − | − | − |
| 40 | 229 R.B. | 184 V | 31.39439 | 073.20733 | + | + | + |
| Year | Location | Galling index | Juveniles/root sample | Juveniles/soil sample | Stylet bearing nematodes | Non-stylet bearing nematodes |
|---|---|---|---|---|---|---|
| 2014 | 134 J.B | 2.20 b | 300.80 b | 140.40 d | 4.20 bc | 2.80 e |
| Moza Rajoya | 3.80 a | 348.60 ab | 280.80 b | 3.80 c | 9.40 cd | |
| Pungu Mor | 2.60 ab | 290.40 b | 108.80 d | 1.60 d | 11.40 bcd | |
| Jamya Abad | 3.20 ab | 390.40 a | 119.00 d | 3.80 c | 12.00 bc | |
| Jandwala | 4.00 a | 297.20 b | 211.40 c | 5.20 ab | 8.40 d | |
| 223 JB-2 | 3.80 a | 336.60 ab | 347.20 a | 5.80 a | 14.00 ab | |
| Rahmuana | 3.20 ab | 294.00 b | 184.00 c | 5.40 ab | 17.20 a | |
| 2015 | 134 J.B | 3.40 a | 172.20 a | 117.80 f | 6.20 cd | 7.20 d |
| Moza Rajoya | 3.20 a | 117.40 c | 242.60 c | 2.80 f | 9.20 cd | |
| Pungu Mor | 2.80 a | 163.20 ab | 136.40 e | 7.40 bc | 13.00 a | |
| Jamya Abad | 3.20 a | 126.40 bc | 135.80 e | 9.20 a | 10.00 bc | |
| Jandwala | 2.80 a | 156.80 abc | 107.00 g | 5.80 de | 10.40 bc | |
| 223 JB-2 | 3.20 a | 134.00 abc | 194.60 d | 4.80 e | 9.20 cd | |
| Rahmuana | 3.60 a | 130.80 abc | 279.60 b | 7.80 b | 11.80 ab | |
| 202 JB | 3.40 a | 131.80 abc | 292.20 a | 7.40 bc | 10.40 bc | |
| 2016 | 134 J.B | 3.40 ab | 278.00 bc | 218.00 b | 5.20 c | 4.00 c |
| Moza Rajoya | 3.20 ab | 268.60 c | 298.80 a | 9.00 a | 10.20 ab | |
| Pungu Mor | 2.80 b | 332.80 abc | 185.20 e | 8.20 ab | 7.20 bc | |
| Jamya Abad | 3.00 b | 349.40 abc | 213.80 bc | 7.40 b | 9.40 ab | |
| Jandwala | 3.40 ab | 380.80 a | 199.20 d | 5.80 c | 8.80 b | |
| 223 JB-2 | 4.20 a | 292.60 bc | 172.60 f | 5.20 c | 9.00 b | |
| Rahmuana | 3.80 ab | 280.80 bc | 211.40 bc | 5.60 c | 6.80 bc | |
| 202 JB | 3.80 ab | 362.00 ab | 204.80 cd | 5.00 c | 8.00 b | |
| 129 JB | 2.80 b | 330.60 abc | 187.20 e | 7.20 b | 12.60 a |
| Year | Location | Galling index | Juveniles/root sample | Juveniles/soil sample | Stylet bearing nematodes | Non-stylet bearing nematodes |
|---|---|---|---|---|---|---|
| 2014 | 58 J.B. | 2.60 b | 334.80 ab | 157.20 e | 5.60 bc | 9.00 c |
| 218 R.B. | 3.60 ab | 352.20 a | 131.60 g | 4.80 cd | 8.80 c | |
| 70 J.B. | 1.40 c | 340.00 a | 219.80 b | 4.80 cd | 11.00 ab | |
| 442 G.B. | 3.60 ab | 332.40 ab | 147.60 f | 4.80 cd | 10.60 abc | |
| 39 G.B. | 3.00 b | 266.20 b | 238.00 a | 6.00 abc | 10.00 bc | |
| 424 G.B. | 2.60 b | 352.60 a | 172.20 d | 6.40 ab | 9.20 bc | |
| 205 R.B. | 3.20 ab | 320.00 ab | 184.00 c | 7.00 a | 12.00 a | |
| UAF | 4.20 a | 280.80 ab | 113.60 h | 4.20 d | 10.40 abc | |
| 2015 | 58 J.B. | 2.60 ab | 336.00 a | 205.60 b | 5.40 cd | 9.20 c |
| 218 R.B. | 2.20 b | 342.20 a | 130.20 e | 5.20 cd | 8.80 c | |
| 70 J.B. | 3.00 ab | 331.00 a | 137.40 e | 4.20 d | 9.80 bc | |
| 442 G.B. | 2.40 ab | 338.40 a | 148.80 de | 5.20 cd | 9.80 bc | |
| 39 G.B. | 3.20 ab | 276.20 a | 185.00 bc | 7.80 a | 10.00 bc | |
| 424 G.B. | 3.80 a | 339.60 a | 128.60 e | 4.80 cd | 9.20 c | |
| 205 R.B. | 2.20 b | 330.60 a | 308.40 a | 7.00 ab | 10.60 abc | |
| UAF | 3.40 ab | 292.60 a | 127.80 e | 5.80 bc | 9.40 bc | |
| 209 R.B. | 2.80 ab | 349.40 a | 172.60 cd | 8.20 a | 11.80 ab | |
| 66 G.B. | 2.60 ab | 352.80 a | 100.40 f | 7.20 a | 13.00 a | |
| 2016 | 58 J.B. | 2.00 d | 361.20 a | 106.80 g | 5.20 de | 9.00 bc |
| 218 R.B. | 2.40 cd | 340.00 ab | 90.60 h | 4.80 de | 9.60 abc | |
| 70 J.B. | 4.00 a | 340.00 ab | 190.80 b | 5.20 de | 10.40 abc | |
| 442 G.B. | 2.20 cd | 328.40 ab | 168.00 c | 9.00 a | 10.20 abc | |
| 39 G.B. | 3.20 bc | 277.80 b | 209.60 a | 5.00 de | 9.80 abc | |
| 424 G.B. | 3.40 ab | 394.00 a | 158.80 d | 7.20 abc | 8.80 bc | |
| 205 R.B. | 2.40 bcd | 362.00 a | 150.60 e | 4.20 de | 8.40 c | |
| UAF | 3.20 abc | 380.80 a | 207.00 a | 6.00 bcd | 9.40 abc | |
| 209 R.B. | 2.80 bcd | 360.40 a | 120.20 f | 5.40 cde | 9.20 abc | |
| 66 G.B. | 3.40 ab | 368.60 a | 162.60 d | 7.60 ab | 10.80 ab | |
| 71 G.B. | 2.60 bcd | 358.00 a | 123.20 f | 3.60 e | 11.20 a |
| Sr # | Local name | Botanical name | Juveniles /root sample | Juveniles/soil sample | Stylet bearing nematodes | Non-stylet bearing nematodes |
|---|---|---|---|---|---|---|
| 1 | Della | Cyperus rotundus | 826.6 bc | 145.6 b | 11.2 de | 6.6 b |
| 2 | Madhana Grass | Dactyloctenium aegyptium | 700.8 cd | 100.0 de | 11.2 de | 4.4 cd |
| 3 | Barnyard grass | Echinochloa crusgalli, | 4914.6 a | 424.0 a | 29.6 a | 9.4 a |
| 4 | False Daisy | Eclipta alba | 646.0 d | 100.6 de | 22.4 b | 6.4 bc |
| 5 | Knotgrass | Paspalum distchum | 494.2 e | 91.2 e | 14.6 cd | 5.4 bcd |
| 6 | Toothed Dock | Rumex dentatus | 783.8 cd | 121.0 cd | 23.0 b | 4.6 bcd |
| 7 | Jangli gai | Avena fatua, | 776.2 cd | 101.6 de | 18.8 bc | 5.0 bcd |
| 8 | Dumbi Sitti | Phalaris minor | 942.8 b | 129.4 bc | 8.4 e | 4.0 d |
| 9 | Cauliflower | Brassica oleracea | 142.2 f | 43.4 g | 10.6 de | 3.4 d |
| 10 | Coriander | Coriandrum sativum L. | 143.8 f | 85.4 ef | 10.2 de | 3.6 d |
| 11 | Maithi | Trigonella foenum-graecum L. | 178.6 f | 64.4 fg | 7.6 e | 5.2 bcd |
| Location | Elevation | Latitude | Altitude | Isolate | GenBank Accession | Nucleotide |
|---|---|---|---|---|---|---|
| Rajoya | 176 | 31.66198 | 072.97448 | JB1CT | KX757064.1 | 326 bp |
| UAF | 179 | 31.43735 | 073.07427 | JB2 UAF | KX757065.1 | 328 bp |
| 58 J.B | 186 | 31.46937 | 072.99122 | JB3FSD1 | KX757066.1 | 326 bp |
| 218 J.B | 173 V | 31.43074 | 072.97399 | JB3FSD2 | KX757067.1 | 326 bp |
| 442 G.B | 172 V | 31.04441 | 073.00982 | JB3FSD3 | MH057345.1 | 326 bp |
| 424 G.B | 172 V | 31.08084 | 073.14034 | JB3FSD4 | MH057346.1 | 326 bp |
| 205 R.B | 186 V | 31.43253 | 073.23050 | JB3FSD5 | MH057347.1 | 326 bp |
| 70 J.B | 181 V | 31.36304 | 72.909520 | JB3FSD6 | MH057348.1 | 326 bp |